What Type of Symmetry Do Annelids Have? — Bilateral, Built From Repeating Rings
Annelids have bilateral symmetry. A single plane down the middle divides them into mirror-image left and right halves. They have a distinct front (anterior) with the mouth and brain, a rear (posterior) with the anus, a back (dorsal) and a belly (ventral) side. On top of that, their bodies are built from repeated segments, each usually with a matching pair of organs, bristles or appendages. Even fan worms, whose feeding crowns look radial, are bilateral underneath.
Cut an earthworm lengthwise down the middle and you get two matching halves. Cut it any other way and you do not. That single plane is what bilateral symmetry means.
What is bilateral symmetry?
An animal is bilaterally symmetrical when only one plane, the sagittal plane, divides it into two roughly mirror-image halves. That plane runs from the head to the tail and from the back to the belly. Animals built this way have three body axes: an anterior-posterior axis from front to rear, a dorsal-ventral axis from back to belly, and a left-right axis that follows from the other two. Once an animal has a fixed head end and a fixed belly side, its left and right sides are defined automatically, and the two are mirror images of one another.
The alternative is radial symmetry, where many planes passing through a central axis cut the body into matching pieces. Jellyfish, most sea anemones and the polyps of corals are built that way, with the mouth at the centre of one surface. Sponges and placozoans show no consistent symmetry at all. Bilateral animals are grouped in the clade Bilateria, which holds roughly 99% of all animals: more than 32 phyla and about a million described species, including annelids, flatworms, roundworms, mollusks, arthropods, echinoderms and vertebrates. Annelids are textbook members of this group. They are bilaterally symmetrical, triploblastic (built from three embryonic tissue layers) and coelomate (with a fluid-filled body cavity), and their more than 22,000 living species include ragworms, earthworms, leeches and a range of tube-dwelling and burrowing worms.
Bilateral symmetry is always approximate. Every bilaterian has some internal organs that are offset from the midline or present on only one side, as the human heart and liver are. When biologists call annelids bilateral, they mean the overall body plan and the way it develops, not that every part is perfectly mirrored. The interesting questions are how that plan is built, how it combines with the annelids’ other defining feature, segmentation, and where it breaks down.
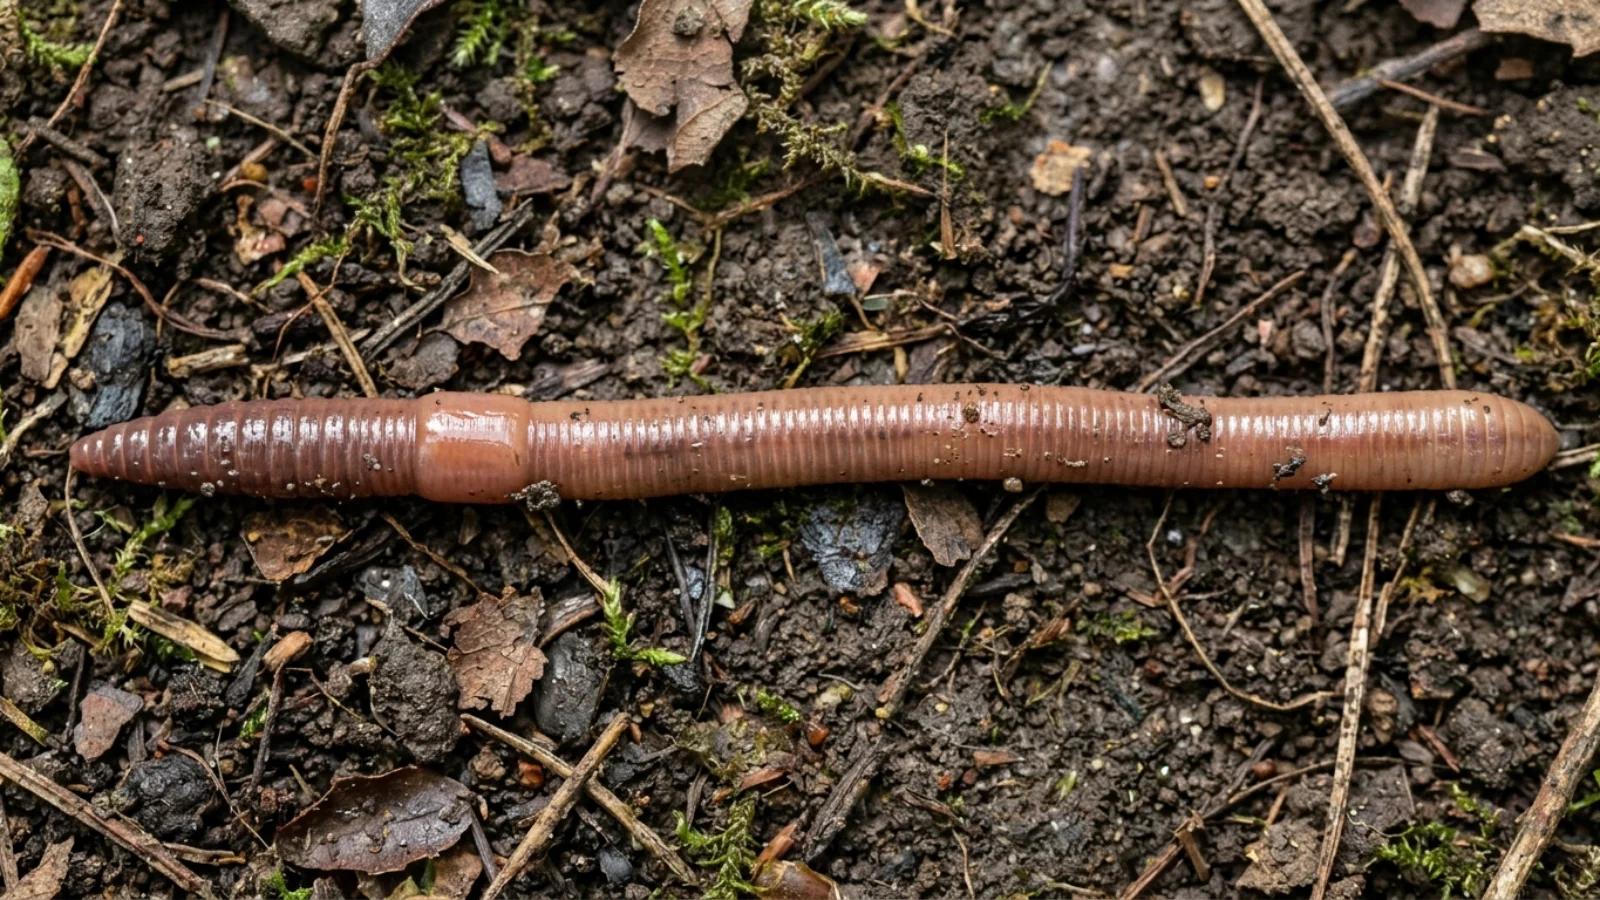
How do annelids show bilateral symmetry?
The outside of a typical marine polychaete makes the plan obvious. At the front is the prostomium, the lobe in front of the mouth, which in most polychaetes carries the brain and paired sense organs such as eyes, antennae and palps. Behind it each body segment carries a pair of parapodia, fleshy lobes that work as legs or paddles, one on the left and one on the right. Each parapodium bears bundles of chaetae, the bristles that give polychaetes (“many bristles”) their name. In the simplest arrangement the chaetae form paired bundles near the top and bottom of each side of every segment, so a cross-section of a ragworm shows four bundles placed symmetrically around the body. At the rear is the pygidium, the tail piece, which carries the anus, generally on the underside.
The inside follows the same pattern. Most annelids have a pair of coelomic cavities in each segment, a left one and a right one. These are separated from neighbouring segments by partitions called septa and from each other by a vertical sheet called the mesentery that runs along the midline above and below the gut. Each segment typically has a pair of nephridia, the excretory organs, one on each side. The nervous system is often described as “ladder-like”: a pair of nerve cords along the belly with a pair of ganglia in each segment, joined by cross-connections like the rungs of a ladder. In most polychaetes the two cords are fused into one, but the paired ganglia remain. Muscles follow suit; beneath the outer circular muscle there are usually four distinct strips of longitudinal muscle.
Structures that are not paired sit on the midline, which is exactly where symmetry predicts they should be. The gut is an almost straight tube from mouth to anus, held in place by the mesenteries. The main dorsal blood vessel runs above it and carries blood forwards, and the ventral vessel runs below it and carries blood backwards. In the earthworm, the connections between them in segments seven to eleven form a pair of aortic arches in each segment that act as hearts, one on each side of the body. The earthworm brain is a pair of pear-shaped cerebral ganglia on the upper side of the gut in the third segment, linked by a pair of connectives running around either side of the pharynx to a pair of ganglia below it. Even the brain, in other words, is a left and right half joined across the middle.
How does segmentation fit with bilateral symmetry?
Annelids layer two kinds of pattern. Along the head-to-tail axis they are segmented, or metameric: the body is a chain of units, each with similar sets of organs. Across each unit they are bilaterally symmetrical. The result is a body that repeats a mirror-image module many times. The name of the phylum comes from the Latin anellus, “little ring”, a reference to those repeated units.
The two ends of the chain are special. Neither the prostomium at the front nor the pygidium at the back counts as a true segment, because neither contains the standard set of organs and neither develops in the same way as the segments between them. New segments form one at a time from a growth zone just in front of the pygidium, so the youngest segment is always at the rear and the oldest is at the front. This pattern is called teloblastic growth. Some annelids, including all leeches, have a fixed maximum number of segments, while others keep adding segments for life. In earthworms the number of segments is usually consistent within a species, and individuals hatch with the number they will keep.
Segmentation interacts with symmetry in a subtle way in the excretory system. The opening through which fluid enters a nephridium lies on the front side of a septum, but the tubule then passes through the septum and its exit pore opens in the following segment. Each nephridium therefore straddles two segments. As a consequence, the first segment has an intake with nothing to discharge it, and the last segment before the growth zone has no intake of its own. The symmetry is left-right, not front-back, and the annelid body is directional from end to end.
Leeches show how external and internal patterns can drift apart. All leech species have 32 segments, or 34 if two specially organised head segments are counted, but the outside of the body is divided into many more narrow rings called annuli. One species has 102. The annuli do not match the internal segments one to one, so a leech looks more finely ringed than it is. Underneath, it is still a bilateral, segmented annelid: the first five segments form the head, with paired eyespots above and a sucker below; 21 mid-body segments each hold a ganglion; and the last seven segments fuse into the rear sucker. Leeches have also lost the septa and the mesenteries that divide most annelid segments into left and right halves, except in the primitive genus Acanthobdella.
Why are annelids bilaterally symmetrical?
Bilateral symmetry suits animals that move steadily in one direction. The front end meets food, mates and danger first, so it pays to concentrate sense organs, a mouth and the main nerve centres there. That trend is called cephalization (the cephalization question has its own page; see the related reading below). A body with a definite front also benefits from being streamlined, which reduces drag in water and makes it easier to push through sediment. A distinct belly gives the animal a surface to grip with, whether that is the bristles of an earthworm or the suckers of a leech. Radial symmetry, by contrast, suits animals that sit still or drift and meet their surroundings equally from every side.
Annelids are a good illustration because their lifestyles cover almost the full range. A crawling ragworm, a burrowing lugworm, a swimming polychaete and an earthworm pushing through soil all travel head first. Even worms that spend their adult lives in tubes descend from mobile ancestors, and the body inside the tube keeps its bilateral plan. During development the anterior-posterior axis is always specified before the dorsal-ventral axis in bilaterians, so the front-to-back direction is the first decision an annelid embryo makes about its own shape.
How does an annelid embryo set up its symmetry?
Annelids belong to the Spiralia, a large group of protostomes that includes mollusks, flatworms and several smaller phyla. The name refers to spiral cleavage, the distinctive way their eggs divide. The first two divisions produce four large cells, labelled A, B, C and D, each of which represents one quadrant of the embryo. Each later division buds off a quartet of smaller cells towards the animal pole at an oblique angle, and the direction of that twist alternates between clockwise and anticlockwise from one quartet to the next. Viewed from above, the cells form a spiral pattern. The early annelid embryo is therefore not bilateral at all: it is organised around a single axis with a built-in rotational twist.
Bilateral symmetry emerges when one quadrant is singled out. In species with equal cleavage, all four large cells look the same at first; after the third quartet forms, one of them makes the most contact with the cells above it and becomes the D quadrant. In species with unequal cleavage, the D cell is larger from the four-cell stage, either because the division spindle is placed off-centre or because a lobe of cytoplasm is shunted into it. Cells of the D quadrant give rise to dorsal and posterior structures, so specifying the D quadrant is what turns a four-part, spirally twisted embryo into one with a back, a belly, and left and right sides.
The molecular signals behind this step differ between annelids. A 2026 study in Nature Communications by Carrillo-Baltodano and colleagues, comparing four annelid species, concluded that in Spiralia the ERK1/2 signalling pathway is the ancestral cue for the posterodorsal side, with the BMP pathway acting downstream of it to promote dorsoventral development. That hierarchy was lost in annelids that switched to unequal cleavage. Capitella teleta uses Activin/Nodal signalling instead, while the ragworm Platynereis dumerilii relies on BMP to set dorsoventral polarity only in the head. The outcome, a bilateral worm, is the same, but evolution has rewired the route to it more than once.
Is the annelid larva bilateral?
Many marine annelids pass through a trochophore larva, a small, top-shaped plankton stage ringed by bands of cilia. At first glance a trochophore looks roughly radial around its long axis, but it is already bilaterally organised, with its mouth on one side of the body rather than at the centre, and its paired structures lie on either side of a midline. When it settles and transforms, the part between its apical tuft and the main ciliary band becomes the prostomium, a small area around the larval anus becomes the pygidium, a band just in front of that becomes the growth zone, and the rest becomes the peristomium, the segment that surrounds the mouth.
The ragworm Platynereis dumerilii, a laboratory model, shows the timing. About 24 hours after fertilisation the egg has become a trochophore, which carries a pair of the simplest eyes known in animals, each made of just one photoreceptor cell and one pigment cell. By 48 hours it is a metatrochophore, and at about 72 hours it becomes a nectochaete larva with three segments, each carrying a pair of parapodia with chaetae. After three to four weeks, when six segments have formed, the head takes shape. At every stage the new structures arrive in left and right pairs. Paired sense organs matter for behaviour too: the pair of larval eyes mediates the larva’s swimming towards light, and adult worms can locate the direction of a chemical cue because it reaches the left and right head cirri at slightly different times.
Why is the annelid nerve cord on the belly?
Annelids, like arthropods, carry their main nerve cord along the belly, below the gut. Vertebrates carry theirs along the back, above it. This difference has long been read as a sign that the vertebrate body plan is an annelid-like plan turned upside down, and molecular work supports the idea that the two are related rather than independently invented. In 2007, Denes and colleagues reported in Cell that the neuroectoderm of Platynereis is subdivided into longitudinal strips by overlapping expression of nk and pax genes. Those strips match the corresponding domains in the vertebrate neural tube, give rise to conserved types of nerve cell and, as in vertebrates, respond to BMP signalling. The authors concluded that this side-to-side architecture was present in the last common ancestor of bilaterians, supporting a single origin of a centralised nervous system. If they are right, the symmetrical layout of an annelid’s nerve cord is a direct inheritance from the ancestor it shares with fish and humans.
Are there annelids that look radially symmetrical?
Yes, in part. Tube-dwelling fan worms spread crowns of feathery tentacles that look like flowers. The best known is the Christmas tree worm, Spirobranchus giganteus, whose two coloured spirals are a favourite subject for reef photographers. The crowns are highly modified prostomial palps, the paired mouth appendages at the head end, and each spiral is made of ciliated, feather-like tentacles called radioles that carry trapped food to the mouth and also work as gills. The worm’s body, roughly 3.8 cm long, stays hidden in a calcareous tube embedded in living coral. Two crowns side by side are the giveaway: they are the left and right halves of one bilateral animal, not two separate radial ones.
Other annelids have arranged tentacles in a ring around the mouth. Peanut worms, the sipunculans, once treated as a separate phylum and now placed within the annelids on molecular evidence, have a retractable front section called the introvert. In one subclass the mouth at its tip is surrounded by 18 to 24 ciliated tentacles; in another the tentacles form an arc above the mouth. Beard worms, family Siboglinidae, carry anywhere from one to more than 200 thin tentacles on a cephalic lobe. A ring of tentacles is radially arranged, but the animal carrying it remains bilateral: siboglinids still have paired chaetae on their rear segments, and sipunculans have a pair of metanephridia opening near the anus, except in two genera that have only one.
Are any annelids asymmetrical?
Several are, in specific features. The clearest example is the operculum of serpulid tube worms, a plug formed from a modified radiole that seals the tube when the worm withdraws. Serpulids, a family of about 300 species, secrete tubes of calcium carbonate, and in many of them only one side carries a functional operculum. In Hydroides, both sides start with an operculum, but one develops into the working plug while the other stays a small rudiment. The biologist Zeleny reported in 1901 that if the functional operculum of Hydroides dianthus is removed, the rudiment on the opposite side grows into a new functional operculum within a few weeks, while a fresh rudiment grows from the stump. In 1933 Yo Okada, working on Hydroides norvegica, found that the rudiment was already fairly large 20 to 30 hours after the operation and in one experiment fully functional after two weeks. He also noted that the right operculum usually grew faster. This “reversible asymmetry” shows that the left-right choice is not fixed: the working operculum appears to suppress its partner, and removing it releases the other side.
Peanut worms show internal asymmetry of a different kind. Their gut runs back from the mouth and then returns forwards, with the downward and upward sections coiled around each other in a double helix. The anus opens in the front third of the trunk rather than at the rear. Spoon worms, the echiurans, have a convoluted gut and a long proboscis that rolls into a scoop. Neither group shows obvious segmentation as adults, yet both retain a bilateral outline, a front and a rear, and a back and a belly.
A broad survey by the biologist A. Richard Palmer, published in the Proceedings of the National Academy of Sciences in 1996, examined 140 inferred evolutionary transitions between symmetry and asymmetry across 11 classes in five animal phyla. He found that asymmetries that appear in the larva more often evolved directly into a fixed left or right bias, while asymmetries that appear after the larval stage more often began as random “either side” states before becoming fixed. The serpulid operculum, which can switch sides in an adult, fits the second pattern: the asymmetry is real but not genetically fixed to one side.
Did annelids lose segmentation but keep their symmetry?
Molecular phylogenies since 1997 have reshaped annelid classification and shown that segmentation is easier to gain and lose than zoologists once thought. Sipunculans and echiurans, both unsegmented as adults, turn out to be annelids that lost their segments; sipunculans even show rudimentary neural segmentation as larvae. Siboglinids are segmented only in the short rear region called the opisthosoma, which has between 5 and 23 segments separated by septa, each with paired chaetae. Bilateral symmetry has survived all of these changes. That contrast says something about which features are deep and which are flexible: segmentation has come and gone within the annelids, but no annelid has abandoned a bilateral body.
The same lesson applies to the old idea that annelids and arthropods are close relatives because both are segmented. The genes that drive segmentation in arthropods do not appear to perform the same role in annelids, and both phyla have close relatives without segments. Annelids are now placed in the Lophotrochozoa, alongside mollusks and brachiopods, while arthropods sit in the Ecdysozoa, the moulting animals. Their shared bilateral symmetry is inherited from the common bilaterian ancestor; their segmentation may well have evolved separately.
How old is the annelid body plan?
Bilateral animals appear in the fossil record towards the end of the Ediacaran period. The first fossil widely accepted as a bilaterian is Kimberella, dated to about 555 million years ago, and the tiny burrowing animal Ikaria wariootia, among the oldest bilaterians identified, has been dated to between 571 and 539 million years ago. Annelids followed in the Cambrian. Phragmochaeta from Sirius Passet in Greenland, about 518 million years old, was described as the oldest known annelid, and the polychaetes Canadia and Burgessochaeta come from the Burgess Shale of Canada, about 505 million years old. Kootenayscolex, a 508-million-year-old annelid from British Columbia, has bristles on its head segment much like those on its body, which suggests that the annelid head began as a specialised version of an ordinary segment. Soft-bodied worms fossilise poorly, but those early specimens already show paired bristles along a bilateral body.
How does symmetry help annelids regenerate?
A body built from repeated, mirror-image modules is well suited to replacing lost parts. Most polychaetes and oligochaetes can regenerate after injury, and two polychaete genera, Chaetopterus and Dodecaceria, can regrow an entire worm from a single segment. Others can regrow a lost head. Annelids are considered the most complex animals able to recover from damage that severe. Leeches are the exception and cannot regenerate. Reef aquarists meet this ability in bristleworms that survive being cut in two, which is one reason the worms are hard to remove from a tank.
How does annelid symmetry compare with other animals?
Flatworms are bilateral but unsegmented, with a single gut opening in most groups. Roundworms are bilateral and unsegmented, with a complete gut. Arthropods are bilateral and segmented, like annelids, but with a moulted chitin exoskeleton and jointed legs. Mollusks are bilateral in origin, though snails twist their bodies during development and coil their shells to one side. Echinoderms are the striking exception: sea stars and sea urchins have five-part radial symmetry as adults, yet their larvae are bilateral, which shows that they descend from bilateral ancestors. Cnidarians, the jellyfish, anemones and corals, are mostly radial, although many sea anemones and some corals have a weak bilateral symmetry defined by a single groove at the mouth called the siphonoglyph.
Two misconceptions are worth correcting. First, the ring pattern of an earthworm does not make it radially symmetrical; the rings mark segments along the length of the body, while the symmetry runs across them. Second, a radial-looking crown does not make a fan worm radial. Look at the animal as a whole and every annelid, from the smallest coiled Spirorbis tube worm, just 2 to 5 mm across, to the longest earthworm, is built on the same plan: one plane, two mirror-image sides, and a body that repeats itself segment after segment.
What type of symmetry do annelids have?
Bilateral symmetry. One plane from head to tail divides the body into mirror-image left and right halves.
Are earthworms radially symmetrical?
No. Their rings mark segments along the body; the body itself is bilaterally symmetrical, with a front, a rear, a back and a belly.
Are annelids segmented and symmetrical?
Yes. The body is a chain of segments, and each segment usually carries matching left and right parapodia, chaetae, nephridia and nerve ganglia.
Are fan worms radially symmetrical?
No. Their feeding crowns look radial, but they are paired head appendages on a bilateral body. A Christmas tree worm’s two spirals are its left and right palps.
Are any annelids asymmetrical?
In specific features. Many serpulid tube worms have one functional operculum on one side, and peanut worms have a gut coiled in a double helix.
Is the annelid larva bilateral?
Yes. The trochophore larva is bilaterally organised and adds paired segments as it grows into a worm.
Do echinoderms and annelids have the same symmetry?
Not as adults. Sea stars and urchins are five-part radial as adults, but their larvae are bilateral, like annelids.
Why is bilateral symmetry useful?
It suits forward movement: senses and the brain gather at the front, the body can be streamlined, and the belly side grips the ground.
- Wikipedia. Annelid; Bilateria; Symmetry in biology; Spiral cleavage; Earthworm; Leech; Sipuncula; Echiura; Siboglinidae; Serpulidae; Spirobranchus giganteus; Platynereis dumerilii.
- Carrillo-Baltodano A.M. et al. (2026). Developmental system drift in dorsoventral patterning is linked to transitions to autonomous development in Annelida. Nature Communications. doi:10.1038/s41467-026-71950-7
- Denes A.S. et al. (2007). Molecular architecture of annelid nerve cord supports common origin of nervous system centralization in Bilateria. Cell 129. doi:10.1016/j.cell.2007.02.040
- Okada Y.K. (1933). Remarks on the reversible asymmetry in the opercula of the polychaete Hydroides. J. Mar. Biol. Assoc. UK 18(2).
- Palmer A.R. (1996). From symmetry to asymmetry: phylogenetic patterns of asymmetry variation in animals and their evolutionary significance. PNAS 93:14279. doi:10.1073/pnas.93.25.14279
- Brusca R.C., Moore W. & Shuster S.M. (2016). Invertebrates, 3rd ed. Sinauer.
Blane Perun has been exploring Earth’s oceans and marine life for over 25 years. Founder of TheSea.Org in 1999, underwater photographer, coral aquaculture pioneer, and explorer of 80+ countries.
About Blane Perun →