What Type of Symmetry Do Flatworms Have? — Left, Right and a Head in Front
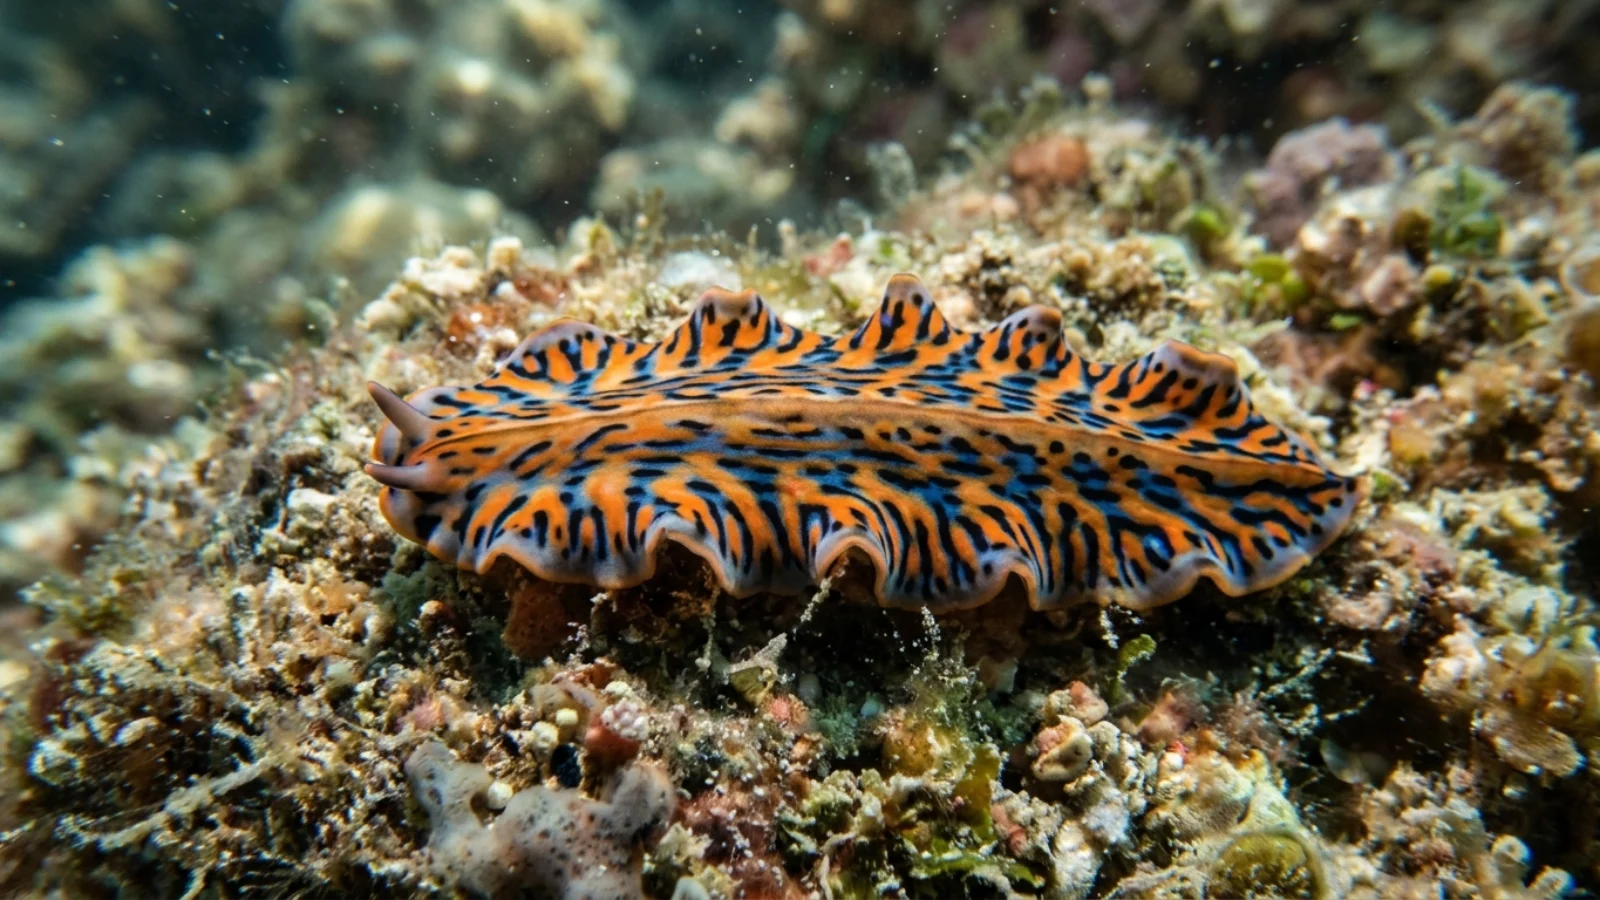
Flatworms have bilateral symmetry. Only one plane, running from head to tail down the middle, divides a flatworm into two mirror-image halves. That gives it a front (anterior) end with a simple brain and eyespots, a rear (posterior), a back (dorsal) side and a belly (ventral) side it crawls on. Bilateral symmetry goes with moving forward head-first, and it led to cephalization, the gathering of nerves and senses at the front, which flatworms show in simple form.
Put a planarian in a dish and it glides off head-first, swinging its front end from side to side as if sniffing the water. That simple behaviour is bilateral symmetry in action: a body with a left and a right side, a head and a tail, a back and a belly, built to travel in one direction.
What is bilateral symmetry?
An animal is bilaterally symmetrical when a single plane, the sagittal or median plane, divides it into left and right halves that are approximately mirror images. Humans, fish, crabs, octopuses and flatworms all share this layout. Any other cut, such as across the body from side to side or from back to belly, produces two halves that are not alike. Once a body has a left and a right, it necessarily also has three axes: an anterior–posterior axis from head to tail, a dorsal–ventral axis from back to belly, and a left–right axis across the width.
Symmetry in biology is always approximate. Folding a leaf in half rarely gives a perfect match, and the same is true of animals. What matters to biologists is the underlying plan: which parts are duplicated, how they are arranged and along which axes the body is organised. By that standard, flatworms are textbook bilaterians. Their left and right sides are mirror images of each other, and, as reference descriptions of the phylum put it, that implies distinct top and bottom surfaces and distinct head and tail ends.
| Term | Meaning in a flatworm |
|---|---|
| Anterior | Head end, with brain ganglia and eyespots |
| Posterior | Tail end |
| Dorsal | Upper side, often patterned in marine species |
| Ventral | Lower side with cilia for gliding, and usually the mouth |
| Lateral | Left and right edges, often ruffled in polyclads |
The flatness of a flatworm is closely tied to this plan. Platyhelminthes have no body cavity and no specialised circulatory or respiratory organs, so oxygen and nutrients must reach every cell by diffusion. A thin, ribbon-like or leaf-like body keeps every cell close to the surface, and many species are microscopic for the same reason. In the larger free-living species the gut is heavily branched, carrying food to all parts of the body. Bilateral symmetry provides the frame; flatness is the engineering solution that lets an animal without lungs or blood vessels grow beyond a few millimetres.
How is flatworm symmetry different from a jellyfish’s?
Jellyfish, sea anemones and corals have radial symmetry. Like a pie, they can be cut into similar slices around a central axis that runs from the mouth on the oral surface to the opposite, aboral end. Radially symmetrical animals have no head and no tail and can meet food or danger from any direction, which suits drifting in open water or sitting fixed to the seabed and waiting for prey to arrive. The French anatomist Georges Cuvier grouped such animals in a branch he called Radiata, a group now recognised as an assemblage of unrelated phyla rather than a natural lineage.
Flatworms take the opposite approach. They move steadily in one direction, so it pays to put the senses and the brain at the leading end and to have a belly specialised for contact with the ground. The difference runs deeper than shape. Flatworms, like all bilaterians, build their bodies from three cell layers, the ectoderm, mesoderm and endoderm, whereas the radially symmetrical cnidarians and ctenophores have only two. The middle layer, mesoderm, gives rise to muscles and organs that make a mobile, directional body possible. The comparison is covered in more detail in cnidarians vs flatworms.
| Feature | Flatworms | Cnidarians |
|---|---|---|
| Symmetry | Bilateral | Radial (or biradial) |
| Head | Yes | No |
| Germ layers | Three | Two |
| Typical lifestyle | Crawling hunters, parasites | Drifting or attached |
The line between the two body plans is not perfectly sharp. The free-swimming planula larvae of some cnidarians show a degree of bilateral symmetry, and one long-standing hypothesis holds that the first bilaterians may have looked rather like such a larva. Many corals and sea anemones also show biradial symmetry, with paired internal structures that create a hint of left and right within an outwardly radial body.
Why is bilateral symmetry important in flatworms?
Because it goes hand in hand with cephalization, the concentration of sense organs and nerve tissue at the front end. Cephalization is a defining feature of most bilaterians, and flatworms show it in a simple, easily studied form. A flatworm’s nervous system has a pair of cerebral ganglia, a simple brain, at the front, connected to longitudinal nerve cords that run down the body joined by cross-connections, a layout often compared to the rails and rungs of a ladder. Some platyhelminths instead have rings of ganglia in the head with main nerve trunks running along the body. See the flatworm nervous system.
The front end carries the sense organs. Most free-living flatworms have pigment-cup ocelli, simple eyes that detect the intensity and direction of light. Most species have one pair, others two or three pairs, and a few large species have many eyes clustered over the brain, mounted on tentacles or spaced around the edge of the body. Chemical sensors are concentrated at the head as well, often on ear-like flaps called auricles in freshwater planarians. That is why a planarian swings its head as it moves: it is sampling chemical gradients on either side and steering toward food.
Bilateral symmetry also makes a muscular, directional body possible. Flatworms glide on a carpet of beating cilia on the ventral surface, riding on a film of mucus, and many can also move by muscular waves running along the body. Marine polyclads add a spectacular third option: some lift off the reef and swim by rippling the left and right margins of the body in waves, steering with the head end. Only an animal with matched left and right edges can swim that way.
Do flatworms have a front and back end?
Yes. In freshwater planarians the anterior end is usually triangular or rounded and often carries auricles and two eyespots. In the hammerhead worms of the genus Bipalium, land planarians native to Asia that have become invasive in the United States, Canada and Europe, the head is broadened into a crescent-shaped head plate; the genus name comes from the Latin for two spades, because the head resembles a pickaxe. In marine polyclads the front often bears a pair of short tentacles, sometimes formed by folds of the body margin.
The mouth is less predictable. Most free-living flatworms have a pharynx that can be everted, turned inside out and pushed out of the body to engulf or digest prey, and the mouth of different species can lie almost anywhere along the underside. In many planarians it sits near the middle of the ventral surface, which surprises people who expect it at the head. The freshwater species Microstomum caudatum can open its mouth almost as wide as its body is long and swallow prey about its own size. These variations do not affect the overall symmetry: the mouth still lies on the midline.
How does a flatworm know which end is its head?
This question has become one of the classic problems of developmental biology, because planarians can regenerate almost any part of the body. Cut a planarian across the middle and the front piece grows a new tail while the back piece grows a new head; split one lengthwise and each half rebuilds the missing side. In the research species Schmidtea mediterranea, almost any fragment can regenerate an entire animal within a few days, thanks to abundant pluripotent stem cells known as neoblasts. Crucially, the new head nearly always forms on the side of the wound that faced forward, so the body somehow remembers its axis.
Research over the past two decades has shown that this memory depends largely on Wnt signalling. Muscle cells near a wound switch on the gene wnt1, which promotes tail formation, while at wounds facing the front, longitudinal muscle fibres switch on notum, a Wnt inhibitor that triggers head regeneration. Studies published in 2025 found that microtubules inside those muscle fibres, and a wound-induced gene called egal-1, help ensure that notum is expressed only at forward-facing wounds; disrupting them can cause head-tail confusion. Genetic screens using RNA interference have identified around 240 genes that affect regeneration in S. mediterranea. Bilateral symmetry in a flatworm is therefore not a fixed shape but an actively maintained pattern, rebuilt from instructions carried in the tissues themselves.
How does symmetry shape a flatworm’s gut and organs?
A bilateral body tends to arrange its organs in pairs either side of the midline, and flatworms follow that pattern. Paired nerve cords run down each side, the excretory system consists of paired networks of fine tubules ending in flame cells, and many species have paired ovaries, testes and eyes. The gut is the main exception to the paired layout but still respects the midline: in planarians, for instance, a single branch runs forward from the pharynx and two branches run backward, one down each side, each with many side pockets.
Most bilaterians, the group sometimes called Nephrozoa, have a through gut running from a mouth at one end to an anus at the other. Flatworms, like the acoels, generally have a bag-like gut with one opening that serves as both mouth and anus. That makes the symmetry of their digestive system unusual among bilaterians, although some long species have evolved an anus, and some with complex, branched guts have more than one. The branching itself is a direct consequence of having no circulatory system: food has to be delivered to every part of a flat, bilaterally arranged body by the gut itself.
Are all flatworms perfectly symmetrical?
Outwardly, close to it; inside and in detail, not always. Reproductive openings, the position of the pharynx and the arrangement of internal organs can be offset slightly from the midline, and the colour patterns of reef polyclads, while broadly mirrored, are rarely exact copies left to right. Biologists accept this: the bilaterian plan describes the organisation of the body, not a perfect geometric reflection.
Parasitic flatworms keep the bilateral plan even in very modified bodies. A tapeworm consists of a scolex, or head, anchored in the host’s intestine by hooks, suckers or both, a short neck, and a strobila, a chain of repeated units called proglottids. The neck produces new proglottids continually, each containing a reproductive tract, and mature ones full of eggs drop off to leave the host. Every unit is bilaterally symmetrical, and the whole animal has a clear front and back. About 6,000 tapeworm species have been described, and probably every vertebrate can host at least one. Flukes, the trematodes, are leaf-shaped and bilateral too, as are the monogeneans that live mainly on the gills and skin of fish.
Were flatworms the first bilateral animals?
They were long taught that way. Because flatworms have no body cavity, they were regarded as a primitive stage in bilaterian evolution, a living model of the earliest animals with a head and tail. Analyses since the mid-1980s have overturned that picture. The acoels and nemertodermatids, once counted as flatworms, have been removed to a separate group, Xenacoelomorpha, which phylogenomic studies place as the sister group of all other bilaterians, although a competing hypothesis links them with echinoderms and acorn worms instead. The remaining true flatworms sit well inside the bilaterian tree, among the protostomes alongside molluscs and segmented worms, and many biologists now think their simple body plan includes losses rather than purely ancestral features.
The fossil record pushes the origin of bilateral symmetry deep into the Ediacaran period. Trace fossils, burrows and trails left by animals moving purposefully through sediment, appear in Ediacaran rocks, and burrows from the Tacuarí Formation of Uruguay are thought to be at least 585 million years old. Kimberella, dated to about 555 million years ago, is widely accepted as an early bilaterian body fossil. In 2020, Scott Evans and colleagues described Ikaria wariootia from the Ediacara Member of South Australia, a tiny organism with a distinct front and back end that matches predictions for the maker of the trace fossil Helminthoidichnites and is one of the oldest bilaterians yet identified. Studies of living animals suggest the common ancestor may have been very small, perhaps around a millimetre long, and simple enough to rely on diffusion as flatworms do. See what phylum are flatworms in?
How does flatworm symmetry compare with other animals?
Symmetry is one of the first features biologists use to sort animal body plans, and only a few types are possible: radial, bilateral, biradial and spherical. Sponges and placozoans show no consistent symmetry at all. Here is where flatworms sit:
| Animal group | Symmetry | Germ layers |
|---|---|---|
| Sponges | None (asymmetrical) | No true tissues |
| Cnidarians (jellyfish, corals) and comb jellies | Radial or biradial | Two |
| Flatworms | Bilateral | Three |
| Echinoderms (sea stars) | Five-part radial as adults; bilateral larvae | Three |
| Vertebrates | Bilateral | Three |
The echinoderms are the instructive exception. Adult sea stars, sea urchins and sea cucumbers show a five-part, or pentaradial, symmetry, but their ciliated, free-swimming larvae are bilaterally symmetrical, and the group evolved from bilateral ancestors. Their radial symmetry is secondary, a later adaptation to a slow-moving or sedentary life on the seabed. Flatworms never went through such a change; from larva to adult, and across free-living and parasitic species alike, they keep the bilateral plan.
That consistency is why flatworms remain a favourite teaching example. In a few millimetres of tissue they show nearly every consequence of bilateral symmetry: a head with a brain and eyes, a belly specialised for movement, paired nerve cords, three germ layers, and the ability to rebuild the whole axis from a fragment. For an overview of the group, see what are flatworms?
What type of symmetry do flatworms have?
Bilateral symmetry: one plane divides the body into mirror-image left and right halves.
Do flatworms have radial symmetry?
No. Radial symmetry is found in cnidarians such as jellyfish and sea anemones.
What is cephalization in flatworms?
The concentration of nerve tissue and sense organs, such as cerebral ganglia and eyespots, at the head end.
How many planes of symmetry does a flatworm have?
One, the sagittal plane running from head to tail down the middle.
Are tapeworms bilaterally symmetrical?
Yes. The scolex and every proglottid in the chain are bilaterally symmetrical.
Do sea stars have the same symmetry as flatworms?
Their larvae are bilateral like flatworms, but adult sea stars have five-part radial symmetry.
Were flatworms the first bilateral animals?
No. Acoel worms, once classed as flatworms, are now placed in a separate group near the base of the bilaterians, and flatworms sit well inside the tree.
How does a regenerating planarian know where to grow a head?
Wound signals in muscle cells decide: the Wnt inhibitor notum switches on at forward-facing wounds and triggers head formation.
- Wikipedia: Flatworm; Planarian; Schmidtea mediterranea; Polycladida; Bipalium; Cestoda; Bilateria; Urbilaterian; Xenacoelomorpha; Echinoderm; Symmetry in biology.
- Evans, S.D. et al. (2020). Discovery of the oldest bilaterian from the Ediacaran of South Australia. PNAS 117. doi:10.1073/pnas.2001045117.
- Miliard, Y. et al. (2025). egal-1 and microtubules promote regeneration polarity in planarians. Development. doi:10.1242/dev.204668.
- Anderson, X.N. & Petersen, C.P. (2025). Planarian microtubules form a network within muscle and regulate injury-induced genes. Development. doi:10.1242/dev.204669.
- Brusca, R.C. et al. (2016). Invertebrates, 3rd ed. Sinauer.
Blane Perun has been exploring Earth’s oceans and marine life for over 25 years. Founder of TheSea.Org in 1999, underwater photographer, coral aquaculture pioneer, and explorer of 80+ countries.
About Blane Perun →